From the free course Introductory Biology on Lykke
DNA Structure and Replication
Key concepts: Nucleotide Structure · Phosphodiester Bonds · DNA Polymerase · Replication Fork · Leading and Lagging Strands
Detailed mechanics of DNA stability, base pairing, and the enzymatic process of replication.
DNA Structure and Replication
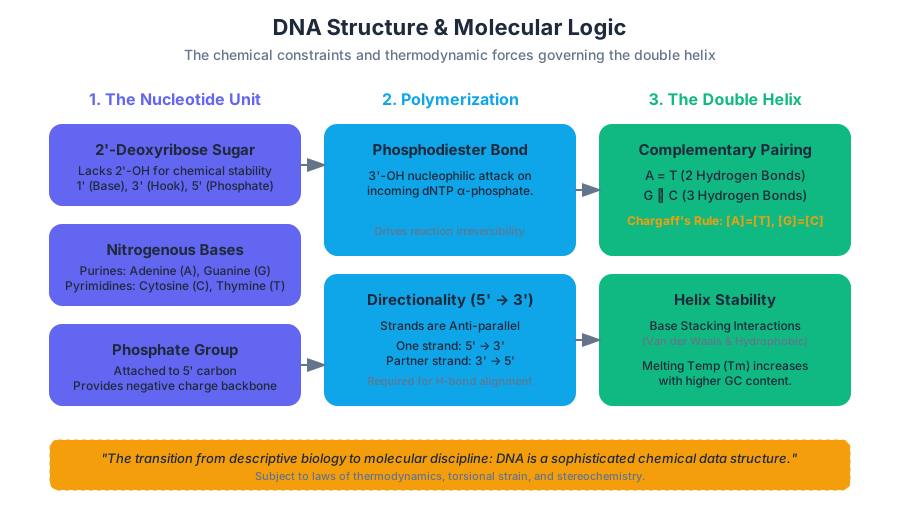
The transition of biology from a purely descriptive science to a rigorous molecular discipline is nowhere more evident than in the study of deoxyribonucleic acid (DNA). As we move from the macroscopic observations of Mendelian genetics to the nanometer-scale interactions of CHNOPS (Carbon, Hydrogen, Nitrogen, Oxygen, Phosphorus, and Sulfur), we find that life’s "blueprint" is not merely a metaphor, but a sophisticated chemical data structure.
In this deep dive, we examine the structural constraints of the double helix and the enzymatic choreography required to replicate three billion base pairs with near-perfect fidelity. We will treat the genome not just as a sequence of letters, but as a physical polymer subject to the laws of thermodynamics, torsional strain, and stereochemistry.
Nucleotide Structure: The Monomeric Unit
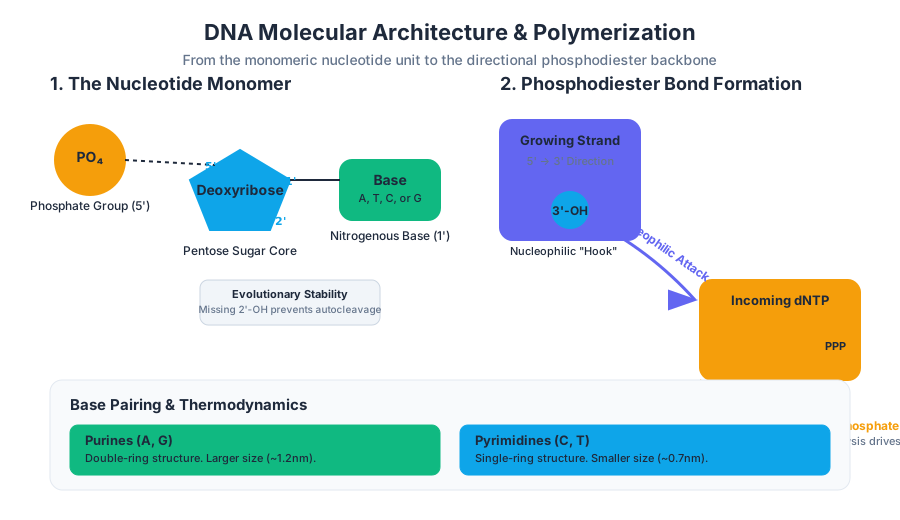
The fundamental building block of the nucleic acid is the nucleotide. To understand DNA, one must first master the anatomy of this monomer. A nucleotide consists of three distinct components: a pentose sugar, a nitrogenous base, and at least one phosphate group.
The Pentose Sugar: Deoxyribose
In DNA, the sugar is 2'-deoxyribose. The numbering of the carbons (1' through 5') is critical for understanding directionality.
- The 1' carbon is the attachment point for the nitrogenous base (via an N-glycosidic bond).
- The 2' carbon is "deoxy" in DNA, meaning it lacks the hydroxyl (-OH) group found in RNA. This single oxygen atom difference is a major evolutionary pivot; the absence of the 2'-OH makes DNA significantly more chemically stable than RNA, as it prevents auto-catalytic cleavage of the phosphodiester backbone.
- The 3' carbon bears a hydroxyl group, which serves as the "hook" for the next nucleotide.
- The 5' carbon is attached to the phosphate group.
Nitrogenous Bases: Purines and Pyrimidines
The "information" in DNA is encoded in the sequence of four nitrogenous bases. These are categorized by their ring structures:
| Feature | Purines | Pyrimidines |
|---|---|---|
| Bases | Adenine (A), Guanine (G) | Cytosine (C), Thymine (T) |
| Structure | Double-ring (6-membered + 5-membered) | Single-ring (6-membered) |
| Size | Larger (~1.2 nm) | Smaller (~0.7 nm) |
| Hydrogen Bond Donors/Acceptors | A: 2 bonds; G: 3 bonds | T: 2 bonds; C: 3 bonds |
The Chargaff Equivalence: In any double-stranded DNA molecule, the amount of A equals T, and the amount of G equals C. This is a direct consequence of the base-pairing requirements dictated by the hydrogen-bonding patterns within the helix.
The Phosphodiester Bond and Directionality
Nucleotides are polymerized into long chains via phosphodiester bonds. This is a covalent linkage where a phosphate group bridges the 5' carbon of one sugar to the 3' carbon of the next.
The Polymerization Mechanism
The synthesis of DNA is an endergonic process driven by the hydrolysis of high-energy nucleoside triphosphates (dNTPs). When a new nucleotide is added, the 3'-OH group of the existing strand performs a nucleophilic attack on the $\alpha$-phosphate of the incoming dNTP. This releases a pyrophosphate (PPi) molecule, which is subsequently hydrolyzed into two inorganic phosphates ($2P_i$). This secondary hydrolysis provides the thermodynamic "push" to make the overall reaction irreversible under cellular conditions.
Anti-parallel Orientation
A DNA double helix consists of two strands running in opposite directions. One strand runs 5' $\rightarrow$ 3', while its partner runs 3' $\rightarrow$ 5'. This anti-parallel nature is not an accident of geometry but a requirement for the hydrogen bonds between bases to align correctly.
Thermodynamics of the Double Helix
The stability of the DNA helix is governed by two primary forces: Hydrogen Bonding between bases and Base Stacking interactions (van der Waals and hydrophobic effects) between the planar faces of the bases.
Melting Temperature ($T_m$)
The $T_m$ is the temperature at which 50% of the DNA molecules in a solution are denatured (separated into single strands). Because G-C pairs share three hydrogen bonds while A-T pairs share only two, DNA with a higher GC content is more thermally stable.
The $T_m$ can be approximated using the Wallace Rule for short oligonucleotides or the more robust nearest-neighbor thermodynamic model for longer sequences.
T_m = \frac{\Delta H}{\Delta S + R \ln(C/4)} - 273.15
Where:
- $\Delta H$: Enthalpy of hybridization
- $\Delta S$: Entropy of hybridization
- $R$: Ideal gas constant
- $C$: Concentration of the DNA
| Interaction | $\Delta H$ (kcal/mol) | $\Delta S$ (cal/mol·K) |
|---|---|---|
| AA/TT | -7.9 | -22.2 |
| AT/TA | -7.2 | -20.4 |
| GC/CG | -9.8 | -24.4 |
| GG/CC | -11.0 | -26.7 |
The Replisome: The Molecular Machine
DNA replication is semi-conservative, meaning each daughter strand consists of one parental template and one newly synthesized strand. This process is executed by the replisome, a complex multi-protein machine.
Key Enzymes and Factors
| Enzyme | Function | Mechanism |
|---|---|---|
| Helicase | Unwinds the helix | Breaks hydrogen bonds using ATP hydrolysis. |
| Topoisomerase | Relieves torsional strain | Cleaves and ligates the sugar-phosphate backbone to prevent supercoiling. |
| Primase | RNA Primer synthesis | Provides a free 3'-OH group for DNA Polymerase to start. |
| DNA Polymerase III | Primary synthesis | Adds dNTPs in the 5' $\rightarrow$ 3' direction. |
| DNA Polymerase I | Primer removal | Replaces RNA primers with DNA (5' $\rightarrow$ 3' exonuclease). |
| DNA Ligase | Nick sealing | Catalyzes phosphodiester bond formation between fragments. |
| SSBs | Strand stabilization | Bind to single-stranded DNA to prevent re-annealing. |
The Replication Fork: Leading and Lagging Strands
Because DNA Polymerase can only synthesize DNA in the 5' to 3' direction, the two anti-parallel template strands present a topological challenge at the replication fork.
The Leading Strand
The template strand running 3' $\rightarrow$ 5' allows for continuous synthesis. Once a single RNA primer is laid down, DNA Polymerase III can follow the helicase indefinitely toward the fork.
The Lagging Strand and Okazaki Fragments
The template strand running 5' $\rightarrow$ 3' cannot be synthesized continuously. Instead, it is synthesized in small, discontinuous stretches called Okazaki fragments (typically 1000–2000 nucleotides in prokaryotes, shorter in eukaryotes).
- Primase synthesizes a short RNA primer.
- DNA Pol III extends the primer until it hits the previous fragment.
- DNA Pol I removes the RNA primer and replaces it with DNA.
- DNA Ligase seals the gap between the fragments.
Worked Example: The Geometry of Synthesis
Imagine a replication fork moving at 1,000 nucleotides per second (typical for E. coli).
- Leading Strand: Synthesis is fluid.
- Lagging Strand: If Okazaki fragments are 1,000 bp long, the cell must initiate a new fragment every second. This requires a highly coordinated "looping" of the lagging strand template (the Trombone Model) so that both the leading and lagging strand polymerases can move physically in the same direction as the replication fork, even though they are synthesizing DNA in opposite chemical directions.
Fidelity and Proofreading
The error rate of DNA Polymerase is approximately 1 in $10^5$ based purely on chemical affinity. However, the actual observed error rate in cells is closer to 1 in $10^{10}$. This 100,000-fold increase in accuracy is due to proofreading.
DNA Polymerase III has 3' $\rightarrow$ 5' exonuclease activity. If an incorrect nucleotide is added, the geometry of the double helix is distorted. The polymerase senses this "wobble," pauses, reverses its direction, and clips out the mismatched base before resuming synthesis.
Theorem of Fidelity: The energy required for proofreading is a trade-off against speed. High-speed replication (like in some viruses) often sacrifices fidelity, leading to higher mutation rates.
Real-World Application: PCR and Sequencing
Our understanding of DNA replication has been weaponized into the most powerful tools in biotechnology. The Polymerase Chain Reaction (PCR) is essentially "replication in a tube," using a heat-stable DNA polymerase (Taq) to amplify specific sequences.
Common Pitfalls and Misconceptions
- The "Start from Scratch" Fallacy: Students often forget that DNA Polymerase cannot start a strand from nothing. It requires a 3'-OH. This is why RNA Primase is essential; RNA polymerases do not require a primer.
- Directionality Confusion: Always remember: DNA is read 3' $\rightarrow$ 5' by the polymerase, but synthesized 5' $\rightarrow$ 3'.
- Ligase vs. Polymerase: Ligase does not add new bases; it only joins the sugar-phosphate backbone of existing fragments.
- Nucleotide: The monomer of DNA, consisting of a deoxyribose sugar, a phosphate, and a nitrogenous base.
- Phosphodiester Bond: The covalent bond linking the 3' carbon of one sugar to the 5' carbon of another.
- Anti-parallel: The arrangement where two DNA strands run in opposite directions (5'-3' and 3'-5').
- Helicase: The enzyme that "unzips" the DNA double helix by breaking hydrogen bonds.
- Okazaki Fragments: Discontinuous segments of DNA synthesized on the lagging strand.
- Exonuclease Activity: The "delete key" function of DNA polymerase that allows for proofreading.
- Topoisomerase: The enzyme that prevents DNA from becoming "over-twisted" (supercoiled) during unwinding.
- Why is the 2' carbon of the ribose sugar significant in the evolution of DNA as the primary genetic material?
- If a DNA molecule has a GC content of 65%, would you expect its melting temperature ($T_m$) to be higher or lower than a molecule with 40% GC content? Why?
- Explain the "Trombone Model" of DNA replication. How does it solve the problem of physical directionality at the fork?
- What would happen to the replication process if DNA Ligase were inhibited?
- Why does DNA synthesis require a primer, whereas RNA synthesis does not?
- Compare the roles of DNA Polymerase I and DNA Polymerase III in E. coli.
Core Objectives:
- Diagram a nucleotide and label the 1' through 5' carbons.
- Explain the energetic basis of DNA polymerization (dNTP hydrolysis).
- Contrast the mechanisms of the leading and lagging strands.
- Identify the specific enzymes involved in the replication fork and their sequential order of action.
- Calculate the complement of a given DNA sequence, maintaining proper 5' to 3' notation.
Advanced Review:
- Research the "End Replication Problem" in eukaryotes and how Telomerase addresses the limitations of the lagging strand.
- Analyze the impact of non-covalent interactions (stacking vs. H-bonding) on the structural integrity of the B-DNA form.
Source Materials
Study Introductory Biology on Lykke
This course page is free to open: signed out, you can read its first two sections, and signing in, on any plan, opens the rest. The free Lykke Chrome extension syncs your own Canvas courses, so ChatGPT, Claude and Muse can answer from your classes and deadlines. It only reads Canvas.
Add the free extensionSign in to open every sectionAll sections of Introductory Biology · Browse more course pages